

Example Of Reduced Hybrid Viability
Introduction
Breeders and researchers akin have been interested in hybridization and introgression betwixt divergent genotypes as the potential driver leading to the ecological divergence of progeny (Rieseberg et al., 2007; Arnold et al., 2012). Conversely, hybridization can sometimes involve a reduced hybrid fettle, such as weakness and/or sterility in F1 and later generations, even in cases of hybridization between members of the same species.
Reduced hybrid viability and/or fertility segregating in Ftwo or later generations are referred to equally hybrid breakdown (HB), in which recessive alleles are necessarily associated. This reproductive barrier has been observed for a long time in both plants and animals (Dobzhansky, 1970; Grant, 1971). Many of the genetic analyses of this barrier have revealed that it is accomplished past a complementary effect between and/or among loci with differentiated alleles, commonly called the Bateson–Dobzhansky–Muller (BDM) incompatibility (Rieseberg and Willis, 2007). HB necessarily involves intrinsic postzygotic reproductive barriers, such as hybrid inviability (including weakness, necrosis, and chlorosis) and hybrid sterility (in the male, female person, or both gametes); therefore, some researchers may not distinguish HB from inviability and sterility in the Fone progeny. All the same, I believe that HB is a convenient nomenclature for reproductive barriers because it implies their underlying genetic basis (i.east., the involvement of recessive alleles).
Recent studies using the Arabidopsis model plant species have provided a amend understanding of HB regarding its molecular mechanisms (Vaid and Laitinen, 2019). Conversely, although rice (Oryza species) is a model ingather, the current understanding of the genetic basis of HB remains limited in this species, probably because HB is not a reproductive barrier in F1 hybrids, in which a higher grain production is expected compared with the parental inbred lines, and probably because inferior plants that segregate in Ftwo and later on generations tin can be easily selected out based on the phenotype from the breeding population. The difficulty in genetic mapping acquired by recessive inheritance can also exist behind this limitation.
Here, I outline HB in rice crosses while referring to information provided by Arabidopsis studies, and discuss how HB is handled in rice breeding.
The Genetic Basis of Hybrid Breakdown in Rice
It is considered that cultivated rice, O. sativa japonica and indica, forms a species complex with their putative progenitor (O. rufipogon) and wild species; however, multiple reproductive barriers, including HB, are observed in crosses among them (Oka, 1988; Vaughan et al., 2003).
To the all-time of my knowledge, Dr. Oka was the get-go to describe the genetic footing of HB in intersubspecific crosses between japonica and indica, which was deemed for by two complementary genes (Oka, 1957). Still, the responsible genes were not mapped on chromosomes, because molecular markers were non bachelor at that time.
In rice hybrids, HB has oft been described in intersubspecific (O. sativa ssp. japonica × ssp. indica) and interspecific (O. sativa × O. nivara and O. sativa × O. glumaepatula) crosses (Oka, 1957; Sato and Morishima, 1988; Wu et al., 1995; Li et al., 1997; Fukuoka et al., 1998, 2005; Kubo and Yoshimura, 2002, 2005; Matsubara et al., 2007a,b, 2015; Yamamoto et al., 2007; Ichitani et al., 2012;for intersubspecific crosses; Sobrizal et al., 2001; Miura et al., 2008 for interspecific crosses) (Table one). Virtually of these HB cases were caused by 2-locus BDM incompatibility and recessive alleles, whereby 1/xvi of the F2 progeny that was homozygous for recessive alleles at both loci showed the HB phenotype; nevertheless, 4/16 of the progeny that was heterozygous at only one locus showed the HB phenotype, depending on the cross combination (Table one and Figure 1A). In the backcross hybrids, 1 locus was already fixed with the alleles from the recurrent parent; therefore, 1/4 of the BCnorthF2 progeny exhibited the HB phenotype (Tabular array 1 and Figure 1B).
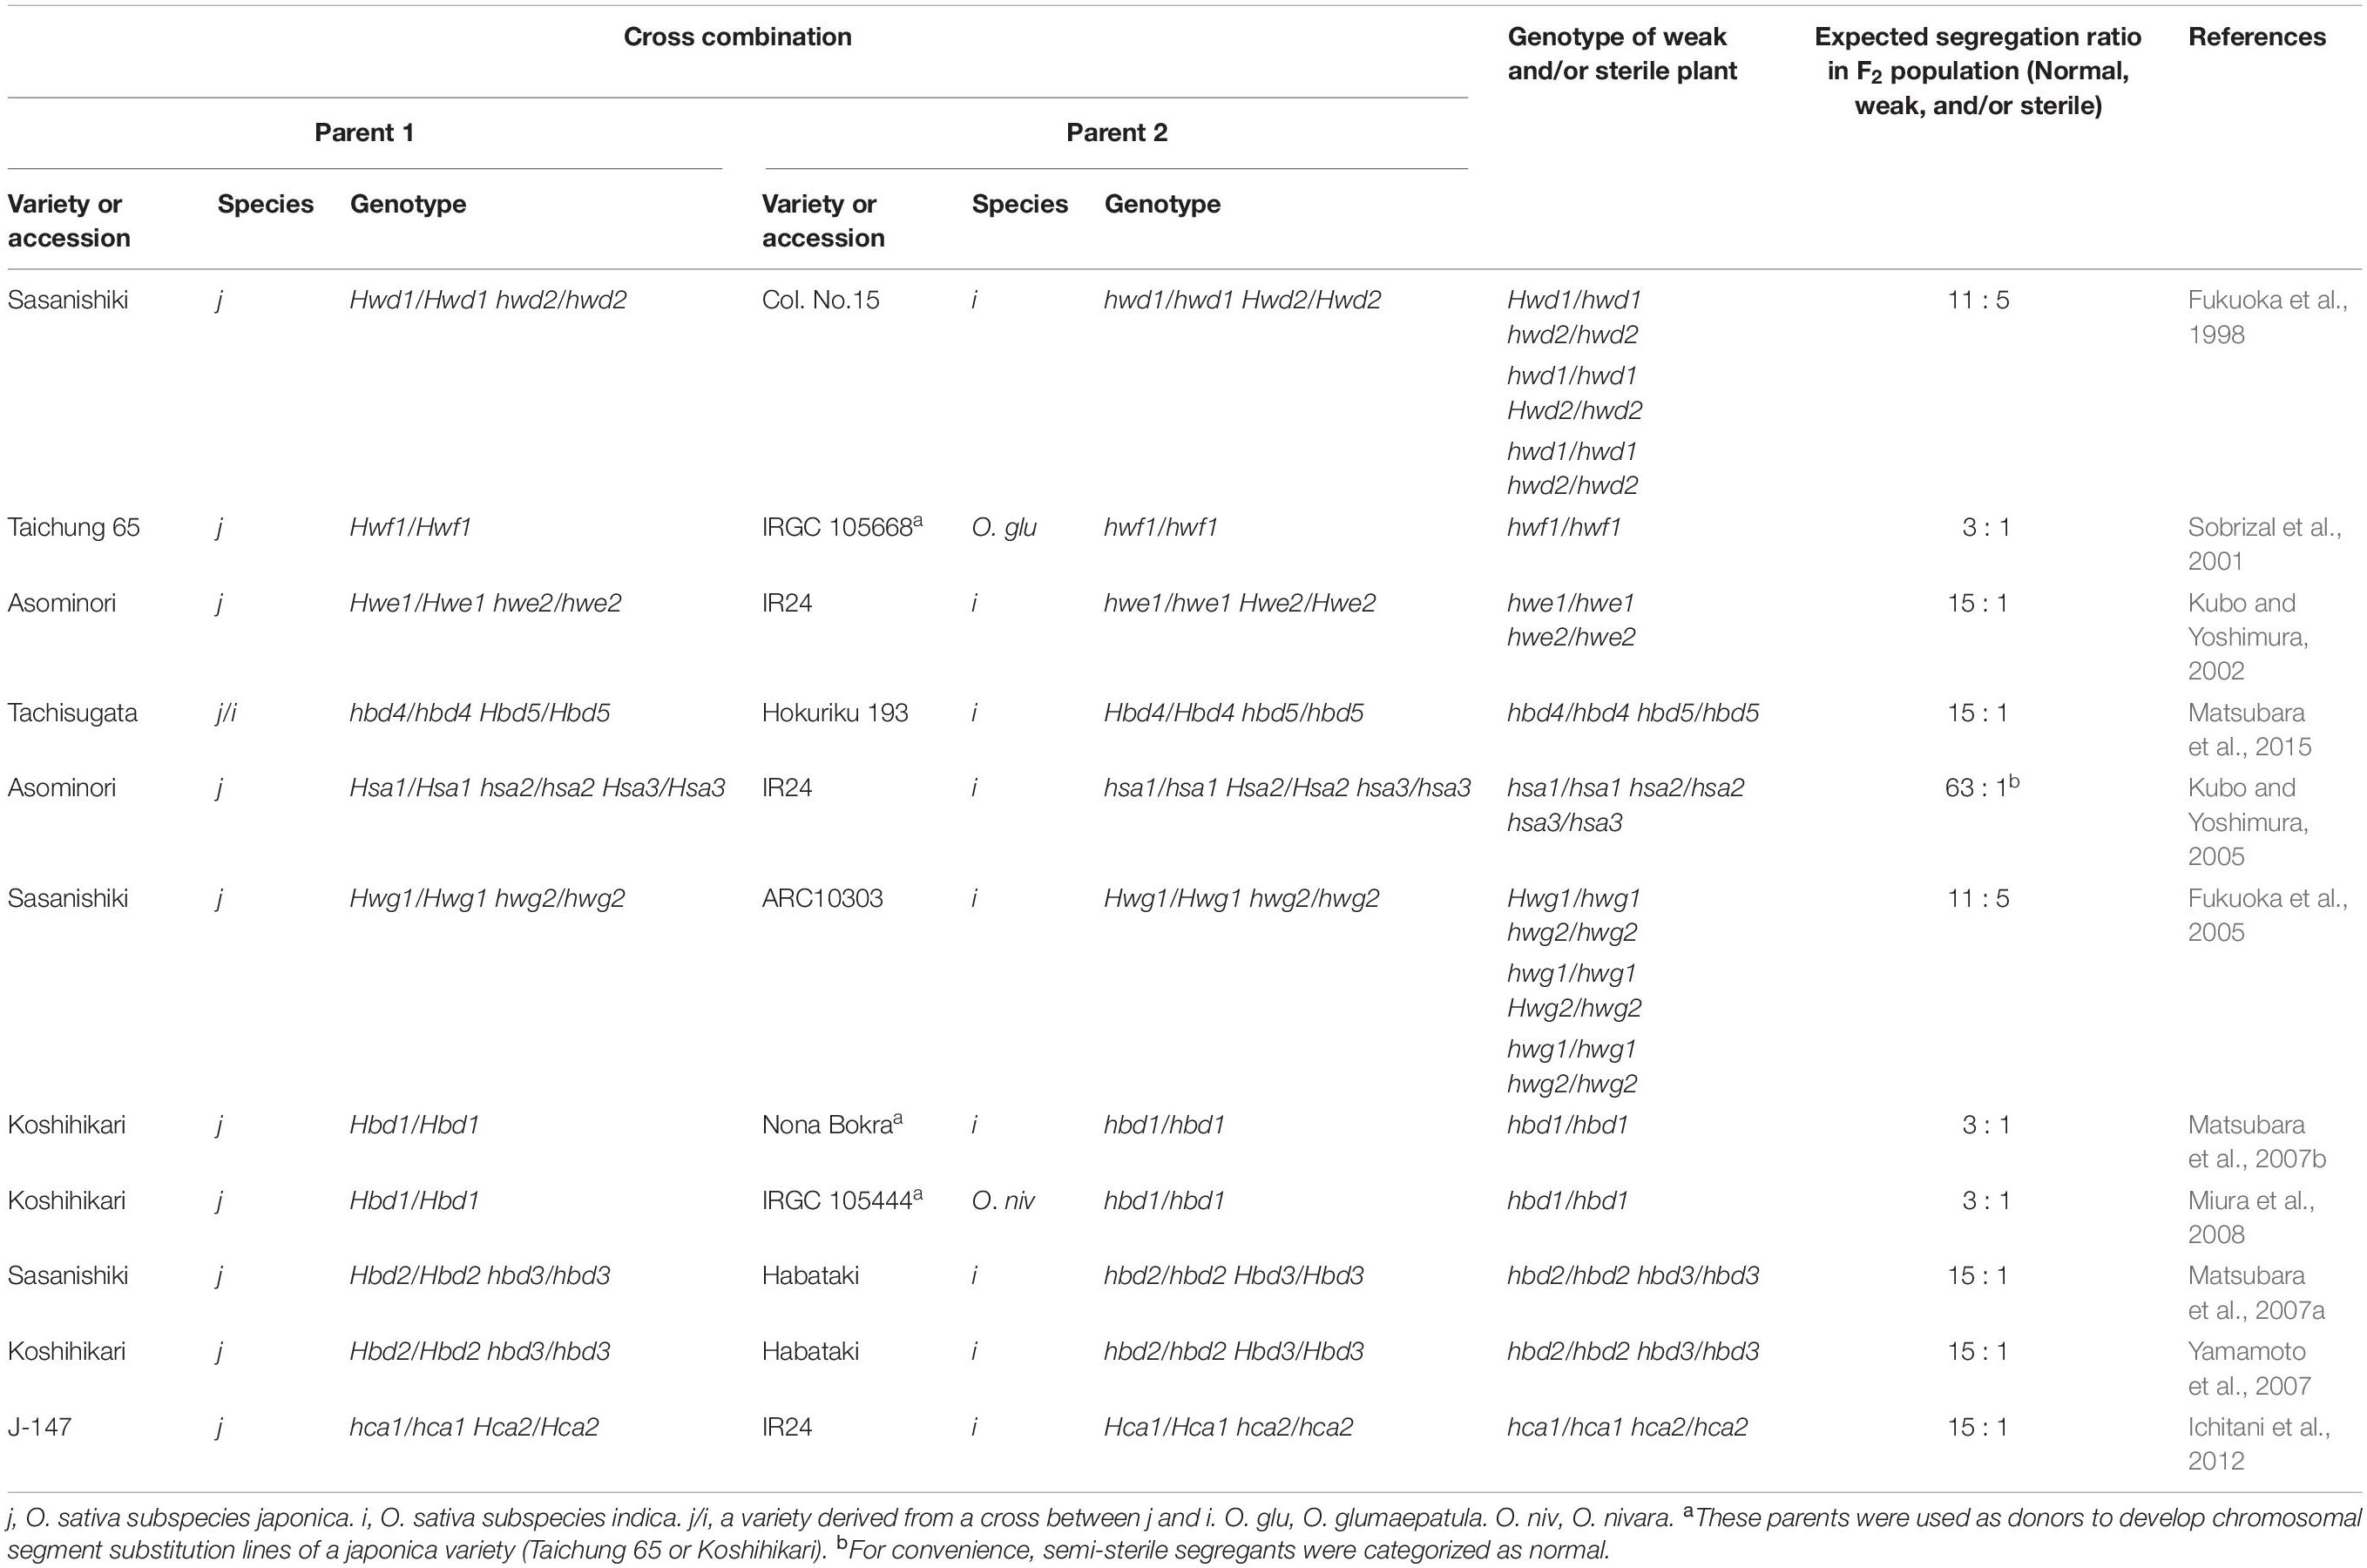
Table i. Genetic basis of the hybrid breakdown reported in rice crosses.
Figure i. The genetic ground of hybrid breakup (HB). (A) Schematic representation of the HB genotype that segregates in the F2 progeny. When the parental genotypes are AAbb and aaBB, i/sixteen of the F2 progeny without dominant allele, which is indicated by grey grapheme (i.east., aabb), bear witness reduced viability and/or fertility, although the other genotypes are normal. In some rice crosses, the F2 progeny with simply one dominant allele (i.e., Aabb, aaBb) also testify reduced viability and/or fertility. (B) Schematic representation of the HB genotype that segregates in the BCnFii progeny. Further, i/iv of the BCnF2 progeny shows reduced viability and/or fertility. (C) Chromosomal location of genes underlying HB in rice crosses. The genes are roughly mapped based on the results of factor mapping in each study. A gear up of complementary genes are connected by the dotted line. Complementary genes with hbd1 and hwf1 have not been reported. The case of the functional nucleotide polymorphism causing HB published by Yamamoto et al. (2010) is shown, and this information will allow u.s.a. to conduct a survey by SNP assortment or amplicon sequencing.
The HB phenotype in rice hybrids varies according to the cross combination. For example, the hbd2/hbd2 hbd3/hbd3 genotype shows weakness, but no obvious seed sterility. However, the hbd4/hbd4 hbd5/hbd5 genotype exhibits both weakness and seed sterility (Matsubara et al., 2007a, 2015; Yamamoto et al., 2007; Table 1). In that location are besides complicated cases in which HB showing both weakness and seed sterility are observed (hwe1/hwe1 hwe2/hwe2 genotype) or HB showing only seed sterility (hsa1/hsa1 hsa2/hsa2 hsa3/hsa3) is found, despite the same cross combination, i.east., Asominori × IR24 cross (Kubo and Yoshimura, 2002, 2005; Table i). Every bit these HBs have independent genetic bases, at least 5/64 of F2 progeny would show the HB phenotype in this cantankerous.
To appointment, several sets of loci responsible for HB have been mapped to particular genomic regions using Dna markers in crosses between the japonica and indica rice varieties (Chrs seven and ten, Fukuoka et al., 1998; Chrs 1 and 12, Wu et al., 1995; Kubo and Yoshimura, 2002; Matsubara et al., 2015; Chrs half dozen and eleven, Fukuoka et al., 2005; Chrs 8, 9, and 12, Kubo and Yoshimura, 2005; Chrs ii and 11, Matsubara et al., 2007a; Yamamoto et al., 2007, 2010; Chrs 11 and 12, Ichitani et al., 2012; Table one and Figure 1C). The results of these studies revealed that loci underlying rice HB are shared in some crosses, but differ in other crosses, which is suggestive of their diversification in rice genomes. For example, in some cases the HB allele carried by O. nivara, a species related closely to incica varieties, share the same locus with an indica variety; however, the HB allele carried past O. glumaepatula, a species closely related to cultivated varieties, does non share the locus with any other diversity (Table 1 and Figure 1C). It should be noted that the HB cases described to a higher place are caused by a set up of genes with major furnishings; still, there are also cases caused by a set of genes with minor effects, eastward.thou., slightly reduced seed fertility, which cannot be overlooked in rice breeding, that have non yet been detected.
Molecular Mechanisms Underlying Hybrid Breakdown
In Arabidopsis hybrids, several molecular mechanisms underlying the BDM type of HB take been experimentally demonstrated, east.g., autoimmune response (Bomblies et al., 2007; Alcázar et al., 2009) and reciprocal silencing of duplicated genes (Bikard et al., 2009; Vlad et al., 2010; Agorio et al., 2017; Blevins et al., 2017).
Autoimmune response: Bomblies et al. (2007) reported starting time that the autoimmune response that an NB-LRR disease-resistance factor or R gene is associated with Arabidopsis HB in intraspecific crosses, although this autoimmune response is mainly expressed as necrosis in F1 plants, and HB in F2 progeny seemed to be conditioned by temperature. In Arabidopsis hybrids, several lines of evidence of HB caused by the autoimmune response accept been described (Alcázar et al., 2009, 2010). The involvement of NB-LRR genes in HB suggests that multiple genomic regions tin be associated with the Arabidopsis HB; in fact, the all-encompassing survey carried out past Chae et al. (2014) supports this idea.
Besides in rice hybrids, HB caused past an autoimmune response has been reported in a japonica × indica cross (Yamamoto et al., 2010). In this case, HB occurs in F2 plants when the hybrid breakup ii (hbd2) gene, which encodes casein kinase I and is carried by the indica variety is combined with a cluster of R genes carried by the japonica diversity. Equally these causative alleles are probable to behave as partially recessive ones, the gene products tin can exist involved (Matsubara et al., 2007a; Yamamoto et al., 2007, 2010).
Reciprocal silencing of duplicated genes: this notion was first theoretically proposed as a genetic basis for hybrid incompatibility (Werth and Windham, 1991; Lynch and Forcefulness, 2000). In the model, i population loses function at i locus and retains it at the other, whereas the other population experiences the opposite result. Consequently, i/sixteen of the Ftwo zygotes do non have functional genes (Lynch and Force, 2000). The HB in Arabidopsis hybrids described by Bikard et al. (2009) and Vlad et al. (2010) is a skilful example of this phenomenon. In this scenario, cases involving epigenetic silencing have also been reported (Agorio et al., 2017; Blevins et al., 2017).
As rice has experienced both whole-genome and segmental duplication (Wang et al., 2007; Guo et al., 2019), reciprocal silencing could be prevalent as a cause of hybrid incompatibility. All the same, to appointment, there is no prove of HB caused past reciprocal silencing of duplicated genes in rice.
Independent of the autoimmune response and reciprocal silencing, an interaction betwixt a DEAD-box RNA helicase 18 and another gene (MORPHEUS MOLECULE 1 every bit a likely candidate) that cause HB in Arabidopsis hybrids has been identified (Plötner et al., 2017; Vaid et al., 2020). Interestingly, the HB phenotype reduces between the Fiii and F4 generations, implying epigenetic regulation of gene expression.
In rice hybrids, among the iii hybrid sterility-a (hsa) loci, Kubo et al. (2016) recently showed that the hsa1 locus consists of 2 genes, and that these genes encode a DUF1618 protein and an uncharacterized protein with some similarity to a nucleotide-binding poly peptide, respectively. The molecular features of the remaining complementary genes, hsa2 and hsa3, have not been reported.
Hybrid Breakdown in Conventional Rice Breeding
For decades, the bulk-population method was widely employed in conventional rice breeding. In this method, later crossing, the F4 or F5 population is raised by cocky-fertilization in bulk (rather than by the single-seed descent method) without artificial pick, but the early generation population is subjected to natural and viability pick (Allard, 1960; Ikehashi and Fujimaki, 1980 for details). In the bulk-population method, many weak and/or sterile genotypes tin be expected to be eliminated from the population earlier the institution of an advanced-generation population; therefore, this method may provide limited information about HB.
For the introgression or accumulation of desirable traits from donor(s) to a variety, rice breeders take often performed backcrossing or multiple parental crossing, followed by the bulk-population method. Empirically, it has long been known that these crossing methods allow the mitigation of the loss of choice candidates by reproductive barriers, because these methods often reduce the segregation of disruptive combinations of alleles associated with HB in a hybrid progeny. Nevertheless, the mitigation of reproductive barriers by these crossing methods is inevitably dependent on the HB genotype of the parents.
Hybrid Breakup in Genomics-Assited Breeding
The publication of reference ingather genome sequences and the evolution of next-generation sequencing technologies take accelerated the progress of the molecular convenance of crops (Kole et al., 2015). In this context, genomics-assisted breeding, such as genomic selection based on genotypes of genome-wide Deoxyribonucleic acid markers, has been considered in ingather breeding (Spindel and Iwata, 2018).
In genomics-assisted breeding of self-pollinated crops, advanced-generation populations, such as recombinant inbred lines, are often used as reference populations, from which genome-broad genotype and phenotype data are obtained. Subsequently, choice based only on marking genotypes is carried out in the progeny of early on generations (east.chiliad., F2). In this selection scheme, information technology should be noted that the reference population does not usually provide the information of genomic region for HB, because weak and/or sterile progeny should have been eliminated in the early generations afterwards crossing. Therefore, if such pick scheme is adopted, we will have to abandon some of import selection candidates. Alternatively, we may select undesirable candidates such that HB becomes credible in later generations.
Give-and-take
Despite the limited number of studies on this subject area, it seems that the loci underlying HB in rice crosses are diversified rather than shared (Table 1 and Figure ane). Every bit described in a higher place, the information on the distribution of HB-associated alleles among cantankerous parents should be a prerequisite for rice breeding, especially for maximizing the effectiveness of genomics-assisted breeding. Therefore, the additional detection of HB in rice crosses and the mapping of responsible genes in the rice genome are needed. In Arabidopsis hybrids, such data near the R genes and their interacting genes has been extensively surveyed (Alcázar et al., 2010, 2014; Chae et al., 2014). The reporting of the hbd2 gene by Yamamoto et al. (2010) in a rice hybrid is a good example of an extensive survey performed using SNP arrays or amplicon sequencing (Figure 1C). The hbd3 and hsa1 genes are also candidates for this type of survey. Somewhen, the evolution of criteria that allow us to predict HB based on the genomic data of the parental lines volition serve as an important tool for genomics-assisted breeding. Fifty-fifty if a causal factor has not been identified as a single gene, closely linked markers, such as single-nucleotide polymorphisms, will be constructive for classifying HB-associated haplotypes, because the linkage disequilibrium of cultivated rice has been estimated to extend to 100–200 kb, although that of wild species (such as O. rufipogon) may extend over several tens of kb (Mather et al., 2007; McNally et al., 2009; Huang et al., 2010). This information will enable the design of a more efficient and effective cantankerous combination.
Bulked segregant analysis followed by next-generation sequencing can be useful for the mapping of HB-associated loci, as well as conventional linkage mapping (such equally quantitative trait locus analysis), because HB segregants often show distinguishable features (most traits such equally plant tiptop, tiller number, and fertility) from normal growth segregants in each cross population. The conquering of imaging information using a digital photographic camera and drone loading may also play an important role in phenotyping in the laboratory and the paddy field. These efforts will provide valuable data not merely to rice breeders, but too to evolutionary biologists.
Furthermore, if an HB-associated allele is identified, gene disruption through ion axle or genome editing may help overcome HB, equally exemplified past F1 hybrid sterility in rice (Koide et al., 2018; Xie et al., 2019).
Data Availability Statement
All datasets presented in this study are included in the commodity/supplementary material.
Author Contributions
The author confirms being the sole contributor of this piece of work and has approved it for publication.
Conflict of Interest
The authors declare that the research was conducted in the absenteeism of whatever commercial or financial relationships that could be construed equally a potential conflict of interest.
Acknowledgments
I would similar to dedicate this paper to the retentivity of Dr. Darshan Brar. He was an eminent rice breeder who vigorously introduced useful genes carried by wild species into cultivars beyond reproductive barriers.
References
Agorio, A., Durand, S., Fiume, East., Brousse, C., Gy, I., Simon, G., et al. (2017). An Arabidopsis natural epiallele maintained by a feed-forrad silencing loop between histone and DNA. PLoS Genet. 13:e1006551. doi: ten.1371/periodical.pgen.1006551
PubMed Abstract | CrossRef Full Text | Google Scholar
Alcázar, R., García, A. 5., Kronholm, I., de Meaux, J., Koornneef, M., Parker, J. E., et al. (2010). Natural variation at strubbelig receptor kinase 3 drives allowed-triggered incompatibilities between Arabidopsis thaliana accessions. Nat. Genet. 42, 1135–1139. doi: ten.1038/ng.704
PubMed Abstract | CrossRef Total Text | Google Scholar
Alcázar, R., García, A. 5., Parker, J. E., and Reymond, M. (2009). Incremental steps toward incompatibility revealed by Arabidopsis epistatic interactions modulating salicylic acid pathway activation. Proc. Natl. Acad. Sci. United statesA. 106, 334–339. doi: ten.1073/pnas.0811734106
PubMed Abstract | CrossRef Full Text | Google Scholar
Alcázar, R., von Reth, M., Bautor, J., Chae, E., Weigel, D., Koornneef, M., et al. (2014). Analysis of a plant complex resistance gene locus underlying immune-related hybrid incompatibility and its occurrence in nature. PLoS Genet. 10:e1004848. doi: 10.1371/periodical.pgen.1004848
PubMed Abstract | CrossRef Full Text | Google Scholar
Allard, R. Westward. (1960). Principles of Plant Breeding. New York, NY: John Wily and Sons, Inc.
Google Scholar
Arnold, M. 50., Ballerini, E. S., and Brothers, A. Northward. (2012). Hybrid fitness, adaptation and evolutionary diversification: lessons learned from Louisiana Irises. Heredity 108, 159–166. doi: 10.1038/hdy.2011.65
PubMed Abstract | CrossRef Full Text | Google Scholar
Bikard, D., Patel, D., Le Metté, C., Giorgi, V., Camilleri, C., Bennett, M. J., et al. (2009). Divergent evolution of indistinguishable genes leads to genetic incompatibilities inside A. thaliana. Science 323, 623–626. doi: 10.1126/science.1165917
PubMed Abstruse | CrossRef Total Text | Google Scholar
Blevins, T., Wang, J., Pflieger, D., Pontvianne, F., and Pikaard, C. South. (2017). Hybrid incompatibility caused past an epiallele. Proc. Natl. Acad. Sci. U.S.A. 114, 3702–3707. doi: 10.1073/pnas.1700368114
PubMed Abstract | CrossRef Full Text | Google Scholar
Bomblies, K., Lempe, J., Epple, P., Warthmann, N., Lanz, C., Dangl, J. L., et al. (2007). Autoimmune response every bit a mechanism for a Dobzhansky-Muller-type incompatibility syndrome in plants. PLoS Biol. 5:e236. doi: x.1371/journal.pbio.0050236
PubMed Abstract | CrossRef Total Text | Google Scholar
Chae, E., Bomblies, K., Kim, S. T., Karelina, D., Zaidem, M., Ossowski, S., et al. (2014). Species-wide genetic incompatibility assay identifies immune genes as hot spots of deleterious epistasis. Cell 159, 1341–1351. doi: 10.1016/j.cell.2014.10.049
PubMed Abstract | CrossRef Total Text | Google Scholar
Dobzhansky, T. (1970). Genetics of the Evolutionary Process. New York, NY: Columbia University Printing.
Google Scholar
Fukuoka, S., Namai, H., and Okuno, Yard. (1998). RFLP mapping of the genes decision-making hybrid breakdown in rice (Oryza sativa Fifty.). Theor. Appl. Genet. 97, 446–449. doi: 10.1007/s001220050915
CrossRef Full Text | Google Scholar
Fukuoka, S., Newingham, 1000. C. V., Ishtiaq, Thousand., Nagamine, T., Kawase, Yard., and Okuno, 1000. (2005). Identification and mapping of two new loci for hybrid breakdown in cultivated rice. Rice Genet. Newslett. 22, 29–31.
Google Scholar
Grant, Five. (1971). Plant Speciation. New York, NY: Columbia University Printing.
Google Scholar
Guo, H., Jiao, Y., Tan, X., Wang, X., Huang, X., Jin, H., et al. (2019). Gene duplication and genetic innovation in cereal genomes. Genome Res. 29, 261–269. doi: 10.1101/gr.237511.118
PubMed Abstruse | CrossRef Total Text | Google Scholar
Huang, 10., Wei, X., Sang, T., Zhao, Q., Feng, Q., Zhao, Y., et al. (2010). Genome-wide association studies of 14 agronomic traits in rice landraces. Nat. Genet. 42, 961–967. doi: 10.1038/ng.695
PubMed Abstract | CrossRef Full Text | Google Scholar
Ichitani, Chiliad., Takemoto, Y., Iiyama, Yard., Taura, S., and Sato, M. (2012). Chromosomal location of HCA1 and HCA2, hybrid chlorosis genes in rice. Int. J. Plant Genomics 2012:649081. doi: 10.1155/2012/649081
PubMed Abstruse | CrossRef Total Text | Google Scholar
Ikehashi, H., and Fujimaki, H. (1980). "Modified bulk population method for rice breeding," in Proceedings of the International Rice Research Conference on Innovative approaches to rice breeding, (Los Baños, PA: International Rice Research Institute), 163–182.
Google Scholar
Koide, Y., Ogino, A., Yoshikawa, T., Kitashima, Y., Saito, Due north., Kanaoka, Y., et al. (2018). Lineage-specific factor acquisition or loss is involved in interspecific hybrid sterility in rice. Proc. Natl. Acad. Sci. U.S.A. 115, E1995–E1962. doi: 10.1073/pnas.1711656115
PubMed Abstract | CrossRef Full Text | Google Scholar
Kole, C., Muthamilarasan, Thousand., Henry, R., Edwards, D., Sharma, R., Abberton, Grand., et al. (2015). Application of genomics-assisted breeding for generation of climate resilient crops: progress and prospects. Front. Found Sci. 6:563. doi: x.3389/fpls.2015.00563
PubMed Abstruse | CrossRef Full Text | Google Scholar
Kubo, T., Takashi, T., Ashikari, M., Yoshimura, A., and Kurata, Due north. (2016). Ii tightly linked genes at the hsa1 locus cause both F1 and F2 hybrid sterility in rice. Mol. Plant 9, 221–232. doi: ten.1016/j.molp.2015.09.014
PubMed Abstract | CrossRef Full Text | Google Scholar
Kubo, T., and Yoshimura, A. (2002). Genetic basis of hybrid breakdown in a Japonica/Indica cross of rice, Oryza sativa L. Theor. Appl. Genet. 105, 906–911. doi: 10.1007/s00122-002-1059-ane
PubMed Abstract | CrossRef Full Text | Google Scholar
Kubo, T., and Yoshimura, A. (2005). Epistasis underlying female sterility detected in hybrid breakdown in a Japonica-Indica cantankerous of rice (Oryza sativa L.). Theor. Appl. Genet. 110, 346–355. doi: 10.1007/s00122-004-1846-y
PubMed Abstract | CrossRef Full Text | Google Scholar
Li, Z., Pinson, South. R. M., Paterson, A. H., Park, W. D., and Stansel, J. Westward. (1997). Genetics of hybrid sterility and hybrid breakdown in an intersubspecific rice (Oryza sativa L.) population. Genetics 145, 1139–1148. doi: 10.1142/9789812814289_0039
CrossRef Full Text | Google Scholar
Mather, M. A., Caicedo, A. Fifty., Polato, N. R., Olsen, K. K., McCouch, S., Purugganan, Yard. D., et al. (2007). The extent of linkage disequilibrium in rice (Oryza sativa 50.). Genetics 177, 2223–2232. doi: ten.1534/genetics.107.079616
PubMed Abstract | CrossRef Full Text | Google Scholar
Matsubara, Yard., Ando, T., Mizubayashi, T., Ito, S., and Yano, Grand. (2007a). Identification and linkage mapping of complementary recessive genes causing hybrid breakdown in an intraspecific rice cantankerous. Theor. Appl. Genet. 115, 179–186. doi: x.1007/s00122-007-0553-x
PubMed Abstract | CrossRef Full Text | Google Scholar
Matsubara, M., Ito, S., Nonoue, Y., Ando, T., and Yano, 1000. (2007b). A novel gene responsible for hybrid breakdown found in a cross betwixt japonica and indica cultivars in rice. Rice Genet. Newslett. 23, 11–13.
Google Scholar
Matsubara, K., Yamamoto, E., Mizobuchi, R., Yonemaru, J.-I., Yamamoto, T., Kato, H., et al. (2015). Hybrid breakdown caused by epistasis-based recessive incompatibility in a cross of rice (Oryza sativa L.). J. Hered. 106, 113–122. doi: 10.1093/jhered/esu065
PubMed Abstruse | CrossRef Full Text | Google Scholar
McNally, Grand. Fifty., Childs, Thou. 50., Bohnert, R., Davidson, R. Thou., Zhao, K., Ulat, Five. J., et al. (2009). Genomewide SNP variation reveals relationships among landraces and modernistic varieties of rice. Proc. Natl. Acad. Sci. UsaA. 106, 12273–12278. doi: ten.1073/pnas.0900992106
PubMed Abstract | CrossRef Total Text | Google Scholar
Miura, K., Yamamoto, E., Morinaka, Y., Takashi, T., Kitano, H., Matsuoka, M., et al. (2008). The hybrid breakdown ane(t) locus induces interspecific hybrid breakup betwixt rice Oryza sativa cv. Koshihikari and its wild relative O. nivara. Breed. Sci. 58, 99–105. doi: ten.1270/jsbbs.58.99
PubMed Abstract | CrossRef Full Text | Google Scholar
Oka, H.-I. (1988). Origin of Cultivated Rice. Tokyo: JSSP.
Google Scholar
Plötner, B., Nurmi, M., Fischer, A., Watanabe, M., Schneeberger, K., Holm, Southward., et al. (2017). Chlorosis caused by ii recessively interacting genes reveals a role of RNA helicase in hybrid breakdown in Arabidopsis thaliana. Plant J. 91, 251–262. doi: 10.1111/tpj.13560
PubMed Abstract | CrossRef Full Text | Google Scholar
Rieseberg, L. H., Kim, S. C., Randell, R. A., Whitney, 1000. D., Gross, B. L., Lexer, C., et al. (2007). Hybridization and the colonization of novel habitats past annual sunflowers. Genetica 129, 149–165. doi: 10.1007/s10709-006-9011-y
PubMed Abstruse | CrossRef Full Text | Google Scholar
Sato, Y. I., and Morishima, H. (1988). Distribution of the genes causing F2 chlorosis in rice cultivars of the Indica and Japonica types. Theor. Appl. Genet. 75, 723–727. doi: 10.1007/BF00265594
CrossRef Full Text | Google Scholar
Sobrizal, T. C., Yasui, H., and Yoshimura, A. (2001). Mapping of a gene for F2 weakness on chromosome 4 of rice. Rice Genet. Newslett. 18, 61–62.
Google Scholar
Spindel, J., and Iwata, H. (2018). "Genomic choice in rice breeding," in Rice Genomics, Genetics and Convenance, eds T. Sasaki and M. Ashikari (Singapore: Springer).
Google Scholar
Vaid, N., Ishihara, H., Plötner, B., Sageman-Furnas, Yard., Wiszniewski, A., and Laitinen, R. A. E. (2020). Leaf chlorosis in Arabidopsis thaliana hybrids is associated with transgenerational reject and imbalanced ribosome number. New Phytol. [Epub ahead of print] doi: 10.1111/nph.16752
PubMed Abstract | CrossRef Full Text | Google Scholar
Vaughan, D. A., Morishima, H., and Kadowaki, Chiliad. (2003). Diversity in the Oryza genus. Curr. Opin. Plant Biol. 6, 139–146. doi: 10.1016/S1369-5266(03)00009-8
CrossRef Total Text | Google Scholar
Vlad, D., Rappaport, F., Simon, M., and Loudet, O. (2010). Gene transposition causing natural variation for growth in Arabidopsis thaliana. PLoS Genet. half dozen:21. doi: ten.1371/journal.pgen.1000945
PubMed Abstract | CrossRef Total Text | Google Scholar
Wang, X., Tang, H., Bowers, J. E., Feltus, F. A., and Paterson, A. H. (2007). Extensive concerted evolution of rice paralogs and the route to regaining independence. Genetics 177, 1753–1763. doi: x.1534/genetics.107.073197
PubMed Abstract | CrossRef Full Text | Google Scholar
Werth, C. R., and Windham, M. D. (1991). A model for divergent, allopatric speciation of polyploid pteridophytes resulting from silencing of duplicate-gene expression. Am. Nat. 137, 515–526. doi: 10.1086/285180
CrossRef Total Text | Google Scholar
Wu, P., Zhang, G., Huang, Due north., and Ladha, J. K. (1995). Non-allelic interaction workout spikelet sterility in an F2 population of indica/japonica cantankerous in rice. Theor. Appl. Genet. 91, 825–829. doi: 10.1007/BF00223887
PubMed Abstract | CrossRef Full Text | Google Scholar
Xie, Y., Tang, J., Xie, Ten., Li, 10., Huang, J., Fei, Y., et al. (2019). An asymmetric allelic interaction drives allele transmission bias in interspecific rice hybrids. Nat. Commun. 10:2501. doi: 10.1038/s41467-019-10488-3
PubMed Abstruse | CrossRef Total Text | Google Scholar
Yamamoto, Due east., Takashi, T., Morinaka, Y., Lin, S., Kitano, H., Matsuoka, M., et al. (2007). Interaction of two recessive genes, hbd2 and hbd3, induces hybrid breakup in rice. Theor. Appl. Genet. 115, 187–194. doi: x.1007/s00122-007-0554-9
PubMed Abstract | CrossRef Full Text | Google Scholar
Yamamoto, E., Takashi, T., Morinaka, Y., Lin, South., Wu, J., Matsumoto, T., et al. (2010). Gain of deleterious office causes an autoimmune response and Bateson-Dobzhansky-Muller incompatibility in rice. Mol. Genet. Genomics 283, 305–315. doi: 10.1007/s00438-010-0514-y
PubMed Abstract | CrossRef Total Text | Google Scholar

Example Of Reduced Hybrid Viability,
Source: https://www.frontiersin.org/articles/10.3389/fpls.2020.575412/full
Posted by: brownbarromempose.blogspot.com
0 Response to "Example Of Reduced Hybrid Viability"
Post a Comment